


Cells Put a Price Tag on Sensing Their World

A cell never senses its environment directly. Instead, it receives a noisy stream of molecular cues—chemical markers binding to receptors, enzymes switching states, and messenger molecules appearing and disappearing. Extracting a meaningful signal from these fluctuations can improve survival, but doing so comes at a cost. Maintaining chemical currents and producing readout molecules consume energy. Giorgio Nicoletti of the Abdus Salam International Center for Theoretical Physics in Italy and his colleagues now show how achieving optimal sensing performance requires a balance between gained information and spent energy [1]. Their key idea is to formulate this balance in terms of quantities that can be estimated from statistical observations rather than from hard-to-measure microscopic forces. The result turns an appealing description based on thermodynamic principles—spend more energy only when it buys useful information—into one based on a concrete biological adaptive strategy, which could be tested in living or synthetic systems.
Noise is ubiquitous on the molecular scale. Receptors randomly bind to and unbind from signaling molecules in the environment, and the downstream “readout” molecules that ultimately dictate the cell’s response are themselves produced and removed through stochastic reactions. For example, a bacterium searching for nutrients senses attractant molecules in its environment through membrane receptors. Receptor activity is relayed by intermediate signaling proteins to downstream readout proteins, which the cell chemically modifies to control its motion. The cell therefore needs to infer nutrient concentrations via a noisy molecular readout. Cells can reduce the uncertainty inherent to noisy signaling, but they incur a cost—slower response speed or increased energy use—by doing so [2, 3]. These trade-offs constrain what a physical system can know about its surroundings and how quickly that knowledge can guide action.
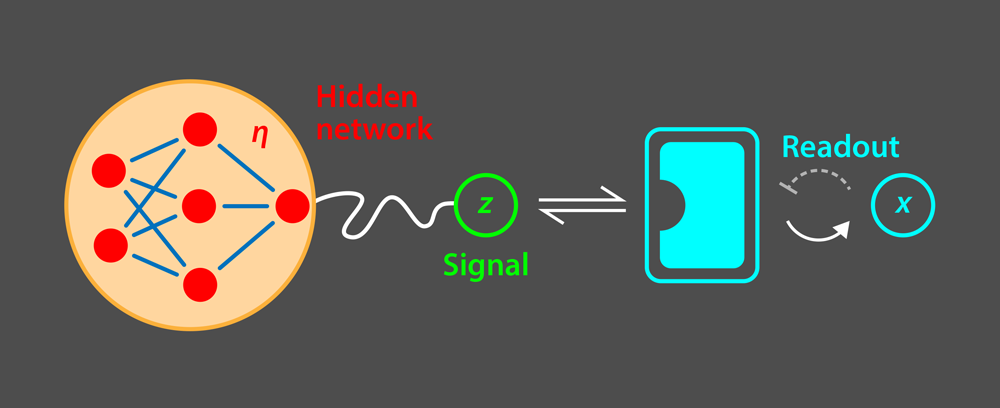
With these trade-offs in mind, evolution could tune a cell’s sensor to be as accurate as possible without spending excessive resources. Imagine that the sensor can tune its response using information about the chemical processes in the signaling network (Fig. 1). But that information is typically incomplete, as some of the chemistry is hidden from the sensor. Stochastic thermodynamics offers a tool kit for quantifying this cost and finding the optimum sensor conditions when a sensing system has complete knowledge of its dynamics—including, for example, the forces driving its fluctuations over time. But this information is typically unavailable. Such incomplete information hence limits the applicability of conventional stochastic thermodynamics methods and requires a new approach that can approximate the true energetic cost.
Nicoletti and colleagues had previously revealed surprising possibilities for how chemical sensors might optimize information harvesting within an energy budget [4]. They found that an observer with access to only part of the system can sometimes harvest more information than one with complete access, although at greater energetic cost. In contrast, an energetically cautious strategy might collect no information at all. Yet this optimization relied on quantities that real chemical and biological sensing machinery cannot readily obtain—thereby assuming more knowledge of the sensing network than a real-world sensor would typically have. The open question became whether a sensor could estimate, from what it can actually observe, both the level of information gained and the energetic cost of sensing. Could the sensor use these estimates to adjust itself when observations are finite and noisy?
The new work addresses this important question in the context of a minimal signaling architecture. Here, a hidden chemical network drives an intermediate signal, which controls the production of a downstream readout molecule. This readout can, in turn, influence the intermediate signal—for instance, by inhibiting its production. In the bacterial sensing example, this coupling regulates how activity in the intermediate signaling proteins gets converted into the downstream readout molecule that controls the bacterium’s motion. Changes in the readout alter this motion and therefore which nutrients the bacterium encounters, feeding back onto receptor activity and the intermediate signal protein. The overall strength of this two-way interaction is adjustable. However, the influence in one direction is not simply balanced by an equivalent influence in the opposite direction. Such asymmetric coupling generally keeps the signal–readout system out of equilibrium and thereby dissipates energy.
Within this asymmetric coupling framework, Nicoletti and colleagues consider a chemical sensor that can adjust its sensing strategy by observing how the intermediate signal and downstream readout fluctuate over time. From these fluctuating trajectories, the sensor estimates how much information the readout contains about the intermediate signal. Crucially, the same observations also provide an estimate of the energetic cost of sensing. The sensor can therefore use experimentally accessible statistics alone to evaluate the trade-off between energy-saving and information-seeking strategies and tune the strength of readout production accordingly. The researchers find that there is a threshold: Below a critical level of preference for information, the optimal response is to switch off signal-driven readout production. Above that value, the optimal production strength increases as information acquisition becomes more important. Remarkably, optimizing the amount of information shared by the observable intermediate signal and readout also increases the information that the readout carries about the internal chemistry of the sensing network.
The conceptual advance is not another statement that biological information has an energetic price. It is an operational bridge between stochastic thermodynamics and evolutionary adaptation. A system need not reconstruct its unobserved reaction dynamics or infer a detailed force field. Rather, observable statistics that describe readily accessible fluctuation trajectories guide changes in sensitivity. This perspective is appealing for biology, where adaptation often occurs through feedback that modifies receptor abundance, enzymatic activity, or gene expression. It could also guide the design of synthetic biochemical circuits and adaptive materials, whose effective strength of signal transmission or feedback can be tuned without requiring complete knowledge of the underlying microscopic reaction networks.
Several steps separate this idea from a true biological mechanism. The conceptualized sensor is an abstract optimizer, and the analysis largely concerns fluctuations near a steady state. A molecular network would need to implement the comparisons through biochemical reactions or adaptive feedback, potentially shaped by evolution. These limitations define an exciting, forward-looking program. First, researchers could identify biochemical motifs that approximate the information-versus-cost trade-off identified in the work. Next, they could test whether measured fluctuation trajectories predict changes in sensitivity. Finally, they could ask whether the same adaptation principle applies when the relevant quantity is not simply the information shared by the signal and readout simultaneously but the readout’s ability to predict future signals or support a particular biological task. More broadly, the study shifts the question from how much information a sensing system contains to how much it can learn via incomplete observations: Which information is truly worth paying for?
References
- G. Nicoletti et al., “Balancing information and dissipation with partially observed fluctuating signals,” Phys. Rev. Lett. 137, 127101 (2026).
- P. R. ten Wolde et al., “Fundamental limits to cellular sensing,” J. Stat. Phys. 162, 1395 (2016).
- G. Lan et al., “The energy–speed–accuracy trade-off in sensory adaptation,” Nat. Phys. 8, 422 (2012).
- G. Nicoletti and D. M. Busiello, “Tuning transduction from hidden observables to optimize information harvesting,” Phys. Rev. Lett. 133, 158401 (2024).